
One man ejaculates into the vagina. Days, hours, or minutes later, a second man can ejaculate into the same vagina while fertilization-capable sperm deposited earlier are still alive inside the cervix, uterus or oviduct. If two ova are released, one man’s sperm can fertilize one ovum and the other man’s sperm the second, producing fraternal twins with different biological fathers.
The phenomenon is called heteropaternal superfecundation. Human cases have been confirmed by forensic DNA testing, and recent reviews describe the phenomenon as rare and difficult to study directly.1, 2
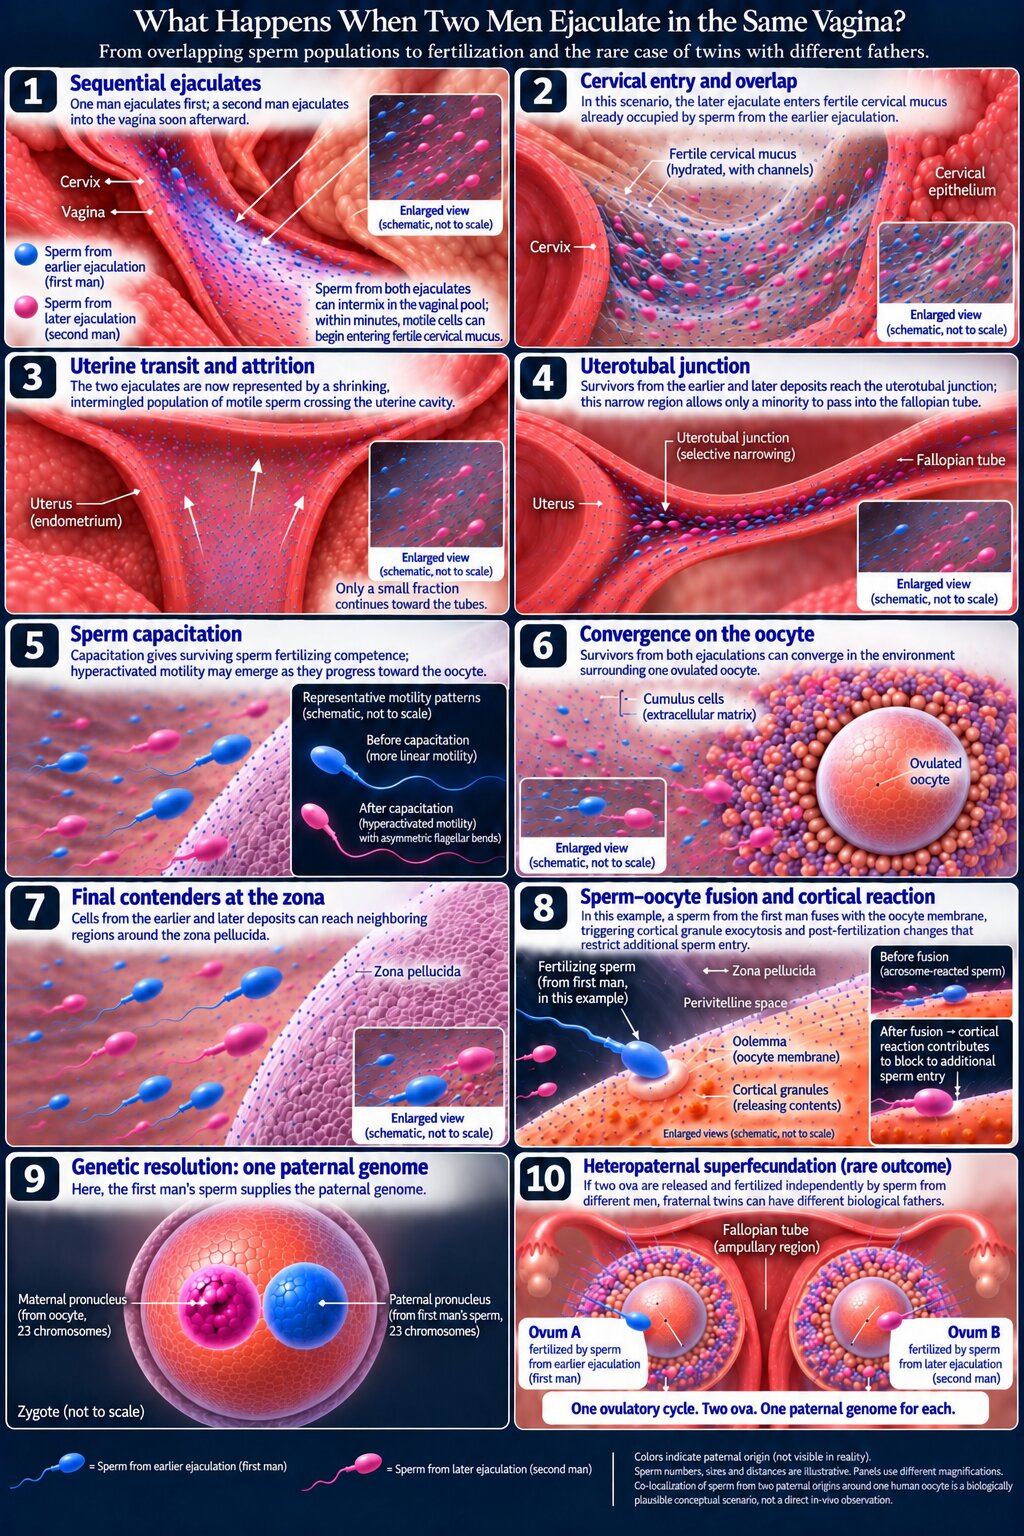
What is heteropaternal superfecundation?
Heteropaternal superfecundation produces dizygotic, or fraternal, twins with different biological fathers.
The exact frequency is difficult to establish because the event is rare, most pregnancies are never tested for multiple paternity, and direct study of atypical human twinning is inherently limited. In a Colombian case published in 2020, autosomal STR and Y-STR testing established different paternity for a pair of male twins. One alleged father matched one twin with a reported probability of paternity of 99.9999%, while numerous genetic markers excluded him as the father of the other twin.3
Can a woman get pregnant by two men during one fertile window?
The event requires two ova and viable sperm from both men during overlapping parts of the fertile window.
Human sperm can enter cervical mucus rapidly after vaginal ejaculation. Classic human postcoital observations reported penetration into cervical mucus within minutes, while contemporary reviews emphasize how strongly transport depends on the female reproductive tract and how difficult natural human transport is to observe directly in vivo.4, 5 If the second ejaculation occurs soon enough, the first man’s sperm may already be inside cervical mucus when the second ejaculate enters the vagina.
What changes if the second ejaculation happens minutes, hours, or days later?
| Time after the first ejaculation | What can be happening biologically | What a second ejaculation means |
|---|---|---|
| First 15 minutes | Progressively motile sperm from the first ejaculation can enter periovulatory cervical mucus within minutes; a human review cites migration into cervical mucus in about 90 seconds.6 | A second man can ejaculate into the vagina while sperm from the first man are already entering the cervix. |
| 15 minutes–2 hours | Human observations place the highest sperm concentration in cervical mucus within this interval.7 | A later ejaculation can deposit fresh semen into the vagina while sperm from the first man are already concentrated in cervical mucus above it. |
| Later the same day | Surviving sperm from the first man may already have passed through cervical selection and moved farther upstream. | Newly deposited sperm from the second man can enter the vagina while older sperm from the first man remain farther inside the reproductive tract. The two paternal populations can occupy different depths of the tract at the same time. |
| 1–5 days later | Fertilization-competent sperm from earlier intercourse can survive into the fertile window. In a prospective cohort, conception occurred after intercourse within a six-day interval ending on the estimated day of ovulation.8 | A second man can ejaculate days later while surviving sperm from the first man remain inside the reproductive tract and may still retain fertilizing capacity. |
What happens when sperm from two men overlap during a fertile window?
1. The first ejaculate starts moving before the second population arrives
After ejaculation, motile sperm begin dispersing from seminal plasma. Human semen usually liquefies within about 30–60 minutes, allowing sperm to swim out of seminal plasma.9 Highly motile sperm can enter cervical mucus much earlier.4, 6 Semen can still be draining out of the vagina while the fastest sperm deposited earlier are already inside cervical mucus. If another man ejaculates during that interval, fresh semen enters below a cervix that may already contain the first man’s sperm.10
If the second ejaculation follows soon afterward, sperm from the first may already be inside cervical mucus while other cells from that ejaculate remain lower in the tract.
2. The later population can enter cervical mucus already occupied by earlier sperm
Around ovulation, cervical mucus becomes highly hydrated and more permissive to sperm transport. Its geometry, viscosity and interaction with motile cells affect which sperm enter the cervix and continue upward.
Sperm differ in progressive motility, morphology, membrane integrity and physiological state, while the female reproductive tract continuously filters the population.4, 5
3. Overlapping populations are reduced to sparse survivors upstream
An ejaculate can contain tens or hundreds of millions of sperm. Only a small fraction enters the cervix, and numbers fall dramatically during transport through the reproductive tract.
4. The uterotubal junction produces another severe narrowing
If survivors from both ejaculations reach the uterus, cells carrying two different paternal genomes face the same narrow uterotubal passage before entering the fallopian tube. Human uterotubal transport is less directly characterized than transport in experimentally studied mammals.4, 5
5. Capacitation changes the surviving sperm
Ejaculated sperm require physiological remodeling before they acquire full fertilizing competence. During capacitation, sperm membrane organization changes, ion fluxes and intracellular signaling shift, and flagellar beating can become hyperactivated—larger, more asymmetric movements associated with fertilizing competence.9, 11
While newly deposited sperm from the later ejaculation are beginning cervical entry, surviving sperm from the earlier man may already be undergoing physiological changes associated with fertilizing competence farther inside the tract.
6. Surviving cells can converge in the environment surrounding one ovulated oocyte
The ovulated oocyte is surrounded by cumulus cells and extracellular matrix. A sperm that reaches the ovulated oocyte still has to traverse the cumulus cells and their extracellular matrix before it can contact the zona pellucida.
If motile sperm from both men survive during overlapping intervals, cells carrying each paternal genome could converge in the environment surrounding one oocyte.2, 4, 9
7. Cells from both populations can become locally interspersed in the cumulus–zona environment
The zona pellucida is the glycoprotein-rich extracellular coat surrounding the oocyte. Human zona pellucida contains ZP1, ZP2, ZP3 and ZP4, and several of these proteins participate in sperm binding and acrosomal physiology.12
Human fertilization research shows that acrosomal exocytosis has a more complex timing than older single-trigger diagrams suggest. Acrosome-reacted sperm can be present within the cumulus, and human zona proteins have distinct roles in sperm interaction.9, 12
Cells carrying two different paternal genomes could therefore be present within the same cumulus–zona environment around one oocyte while remaining genetically distinct.
8. One sperm reaches the oolemma and completes fusion
After traversing the zona pellucida, the fertilizing sperm enters the perivitelline space and reaches the oocyte plasma membrane, or oolemma. Successful fertilization requires molecular recognition and membrane fusion.
IZUMO1 on sperm and JUNO on the oocyte are central components of this recognition system. The IZUMO1–JUNO interaction is conserved across mammals, including humans; its discovery established a molecular receptor pair at the sperm–egg interface.9, 13 The sperm that successfully fuses with the oocyte supplies its paternal genome. IZUMO1–JUNO binding is essential for gamete recognition, although membrane fusion requires additional molecular machinery.
9. Fertilization changes the egg and restricts additional sperm entry
Gamete fusion activates the oocyte and initiates calcium-dependent signaling. Cortical granules, membrane-bound organelles positioned beneath the oolemma, undergo exocytosis and release their contents into the perivitelline space. Their products contribute to post-fertilization changes in the zona pellucida and other mechanisms that restrict additional sperm entry.9, 14, 15 Once a sperm from either man has fused with the oocyte, these changes help restrict entry by additional sperm from either ejaculate.
10. One paternal genome remains in the zygote
The fertilizing sperm contributes one haploid paternal genome. The oocyte completes meiosis, and maternal and paternal pronuclei form before the first mitotic division.
If the fertilizing sperm came from the first man, sperm from the second man contribute no DNA to that embryo; the converse outcome can also occur. If a second ovum is present during the same fertile interval, surviving sperm from the other man can still participate in a separate fertilization event.
Does human sperm competition really happen?
In evolutionary biology, sperm competition describes competition between sperm from two or more males over fertilization opportunities.16
In humans, ejaculates from different men can remain capable of contributing to fertilization during overlapping fertile intervals; detailed competitive interactions between those populations have not been observed directly in vivo.
How long does sperm take to reach the egg?
There is no single human transit time from ejaculation to fertilization. Human postcoital observations show that sperm can enter cervical mucus rapidly, while successful fertilization depends on subsequent transport, timing relative to ovulation and acquisition of fertilizing competence.4, 5 A 2025 review of human sperm navigation describes rheotaxis, thermotaxis and chemotaxis as complementary guidance mechanisms while emphasizing that their in-vivo roles in humans remain incompletely resolved.17
Can two sperm fertilize one egg?
Normal human fertilization is monospermic: one sperm supplies the paternal haploid genome. Pathological dispermy can occur when two sperm contribute to one oocyte, producing an extra paternal chromosome set and a diandric triploid conception.18 Triploidy is a severe chromosomal abnormality commonly associated with pregnancy loss and abnormal development.
Post-fertilization modifications of the mammalian egg coat and plasma membrane contribute to limiting additional sperm entry; the molecular details involve several mechanisms rather than a single barrier.9, 15
Heteropaternal superfecundation follows a separate mechanism: two ova undergo independent fertilization events, with one paternal contribution to each ovum.
How can twins have different fathers?
If two ova are released during one ovulatory period, the first fertilization event does not settle paternity for the second ovum. One ovum can be fertilized by sperm from the earlier man and the other by sperm from the later man. Each event produces its own zygote and its own paternal genotype, so the resulting dizygotic twins can have different biological fathers.2, 3
What determines which man’s sperm fertilizes the egg?
For an actual pregnancy involving two possible fathers during the fertile window, intercourse timing can estimate plausibility. Paternity testing establishes biological fatherhood.
Can ultrasound show that twins have different fathers?
No. Ultrasound can characterize a twin pregnancy, while biological paternity requires DNA testing of each twin and the possible fathers.
Does each twin need separate paternity testing?
Yes. Dizygotic twins arise from separate fertilization events, so paternity must be established for each twin independently. Confirmed heteropaternal cases have done exactly this with DNA marker testing.2, 3
References
- McNamara HC, Kane SC, Craig JM, Short RV, Umstad MP. A review of the mechanisms and evidence for typical and atypical twinning. Am J Obstet Gynecol. 2016;214(2):172–191. doi:10.1016/j.ajog.2015.10.930. ↩
- Timasheva Y, Tuktarova I. Heteropaternal superfecundation in dizygotic twins: a case report and literature review. Forensic Sci Med Pathol. 2025;21(4):1779–1786. doi:10.1007/s12024-025-01046-z. ↩
- Mogollón F, Casas-Vargas A, Rodríguez F, Usaquén W. Twins from different fathers: A heteropaternal superfecundation case report in Colombia. Biomédica. 2020;40(4):604–608. doi:10.7705/biomedica.5100. ↩
- Suarez SS, Pacey AA. Sperm transport in the female reproductive tract. Human Reproduction Update. 2006;12(1):23–37. doi:10.1093/humupd/dmi047. ↩
- Miller DJ. Sperm in the Mammalian Female Reproductive Tract: Surfing Through the Tract to Try to Beat the Odds. Annu Rev Anim Biosci. 2024;12:301–319. doi:10.1146/annurev-animal-021022-040629. ↩
- De Jonge C. Biological basis for human capacitation—revisited. Human Reproduction Update. 2017;23(3):289–299. doi:10.1093/humupd/dmw048. ↩
- Fordney-Settlage D. A review of cervical mucus and sperm interactions in humans. Int J Fertil. 1981;26(3):161–169. ↩
- Wilcox AJ, Weinberg CR, Baird DD. Timing of sexual intercourse in relation to ovulation. Effects on the probability of conception, survival of the pregnancy, and sex of the baby. N Engl J Med. 1995;333(23):1517–1521. doi:10.1056/NEJM199512073332301. ↩
- Chang HY, Gierke T, Tang S, Lu Y. Molecular interplay between sperm and oocyte: a narrative review. Human Reproduction Update. 2026;32(4):409–439. doi:10.1093/humupd/dmag008. ↩
- Practice Committee of the American Society for Reproductive Medicine and the Practice Committee of the Society for Reproductive Endocrinology and Infertility. Optimizing natural fertility: a committee opinion. Fertil Steril. 2022;117(1):53–63. doi:10.1016/j.fertnstert.2021.10.007. ↩
- Puga Molina LC, Luque GM, Balestrini PA, et al. Molecular Basis of Human Sperm Capacitation. Front Cell Dev Biol. 2018;6:72. ↩
- Gupta SK. Human Zona Pellucida Glycoproteins: Binding Characteristics With Human Spermatozoa and Induction of Acrosome Reaction. Front Cell Dev Biol. 2021;9:619868. ↩
- Bianchi E, Doe B, Goulding D, Wright GJ. Juno is the egg Izumo receptor and is essential for mammalian fertilization. Nature. 2014;508(7497):483–487. doi:10.1038/nature13203. ↩
- Liu M. The biology and dynamics of mammalian cortical granules. Reprod Biol Endocrinol. 2011;9:149. ↩
- Fahrenkamp E, Algarra B, Jovine L. Mammalian egg coat modifications and the block to polyspermy. Mol Reprod Dev. 2020;87(3):326–340. doi:10.1002/mrd.23320. ↩
- Parker GA. Conceptual developments in sperm competition: a very brief synopsis. Philos Trans R Soc Lond B Biol Sci. 2020;375(1813):20200061. doi:10.1098/rstb.2020.0061. ↩
- Eisenbach M. Sperm navigation in humans: a concerted action of multiple means. Commun Biol. 2025;8(1):923. doi:10.1038/s42003-025-08358-4. ↩
- McFadden DE, Jiang R, Langlois S, Robinson WP. Dispermy—origin of diandric triploidy: brief communication. Human Reproduction. 2002;17(12):3037–3038. doi:10.1093/humrep/17.12.3037. ↩